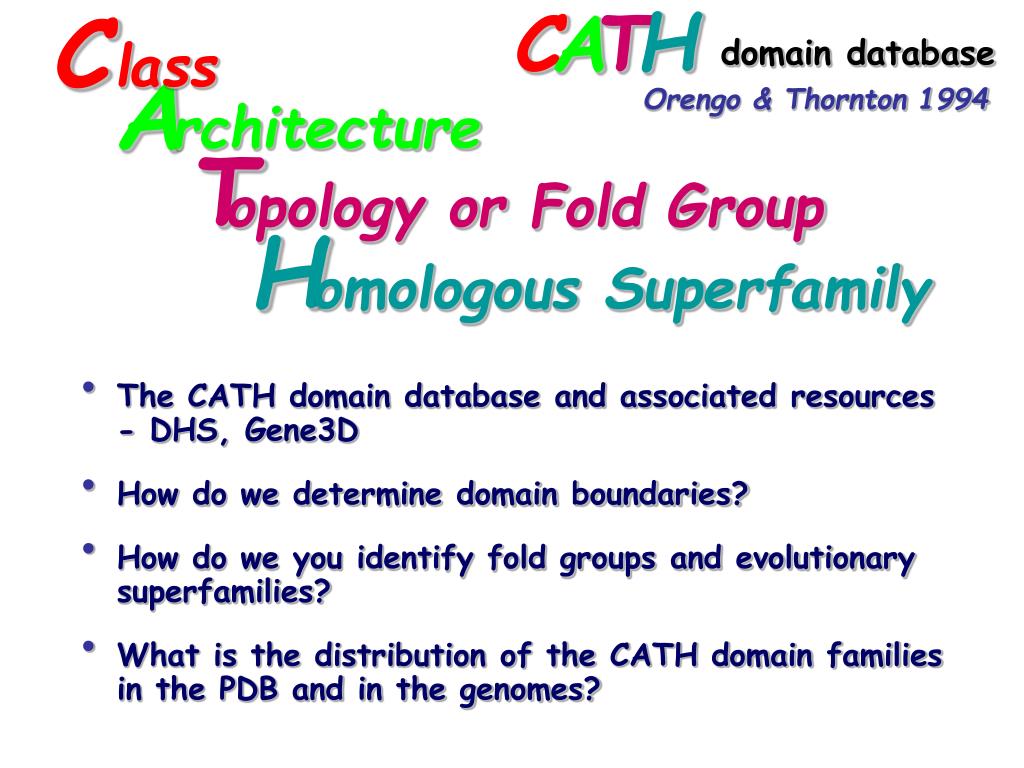
C. H. C. A. T. The CATH domain database and associated resources - DHS, Gene3D How do we determine domain boundaries? How do we you identify fold groups and evolutionary superfamilies? What is the distribution of the CATH domain families in the PDB and in the genomes?. lass.
Une image / un lien ci-dessous est fourni (tel quel) pour télécharger la présentation
Politique de téléchargement : le contenu du site vous est fourni TEL QUEL pour votre information et votre usage personnel ; il ne peut être vendu, concédé sous licence ni partagé sur d’autres sites sans l’accord de son auteur.Le contenu vous est fourni TEL QUEL, pour votre information et votre usage personnel uniquement.Téléchargez la présentation en cliquant sur ce lien.Lors du téléchargement, si vous ne parvenez pas à télécharger une présentation, l’éditeur a peut-être supprimé le fichier de son serveur.Pendant le téléchargement, si vous ne parvenez pas à obtenir une présentation, le fichier a peut-être été supprimé par l’éditeur.
F I N
Plus de contenu associé
Transcription de la présentation
C H C A T The CATH domain database and associated resources - DHS, Gene3D How do we determine domain boundaries? How do we you identify fold groups and evolutionary superfamilies? What is the distribution of the CATH domain families in the PDB and in the genomes? lass domain database A Orengo & Thornton 1994 rchitecture T opology or Fold Group H omologous Superfamily
Multidomain proteins ~20,000 chains from Protein Databank (PDB) ~50,000 domains in CATH structure database ~40% of the entries in CATH are multidomain
Carboxypeptidase A (2ctc) Carboxypeptidase G2 (1cg2A) ~30% of multidomains in CATH are discontinuous
DETECTIVE Swindells 1995 each domain should have a recognisable hydrophobic core DOMAKSiddiqui & Barton, 1995 residues comprising a domain make more internal contacts than external ones PUUHolm & Sander, 1994 parser for protein folding units: maximal interaction within domains and minimal interaction between domains Algorithms for Recognising Domain Boundaries Consensus is sought between the three methods – on average this occurs about 20% of the time
74% Close homologues 29% 21% Twilight zone 4% Midnight zone 11% Homologues/analogues
Sequence Based methods close homologues – BLAST (Altschul et al.) - SSEARCH (Smith & Waterman) remote homologues – SAM-T99 (Karplus et al) Structure Based Methods close & remote homologues - CATHEDRAL (Harrison, Thornton Orengo) - SSAP (Taylor & Orengo) - CORA (Orengo) Algorithms for Recognising Homologues
74% Close homologues SSEARCH 29% 21% Twilight zone HMMs, SSAP 4% Midnight zone CATHEDRAL, SSAP 11% Homologues/analogues CATHEDRAL, SSAP
Hidden Markov Models (HMMs) SAM-T99 Karplus Group SAMOSA Orengo Group Non redundant GenBank database query sequence hits these methods can currently identify ~70% of remote homologues (3 times more powerful than BLAST)
Percentage of PDB structures classified in CATH by different methods over the last 2 years remote homologues (8.6) analogues (1.9) SSAP Novel folds 2.0 1.9 remote homologues (<30%) HMMs 8.6 7.6 20.7 59.2 Close homologues (>30%) SSEARCH Near-identical SSEARCH
7.7 11.8 8.0 22.0 28.4 22.0 Percentage of structural genomics PDB structures classified in CATH by different methods over the last 2 years near-identical SSEARCH novel folds analogues SSAP close homologues (>30%) SSEARCH remote homologues SSAP remote homologues (<30%) HMMs
ignore the variable loop regions and only compare the secondary structures derive vectors through secondary structure elements compare closest approach distances and vector orientations using graph theory Fast Structure Comparison Method (CATHEDRAL) Andrew Harrison et al., JMB, 2002
d a b a . b = | a || b | cos + dihedral angle +chirality
Using CATHEDRAL to Identify Domain Boundaries Graph based secondary structure comparison is very fast - 1000 times faster than residue based methods New multi-domain structures can be rapidly scanned against the library of CATH domains. E-values can be used to identify significant matches. 85-90% of domains in new multi-domain structures have relatives in CATH
CATHEDRAL Multi-domain structure Secondary structure match by graph SSAP residue alignment residues in new multi-domain residues in CATH domain family 1 Fold A residues in CATH domain family 2 Fold B
SSAP Protein A Protein B Taylor & Orengo, J. Mol. Biol. 1989 residue based structure comparison method using dynamic programming Scores range from 0-100 Residues in protein A Residues in protein B
CATHEDRAL One third of known multi-domain structures are discontinuous
Divergence - similarity arises due to divergent evolution from a common ancestor - structure much more highly conserved than sequence Convergence - similarity due to there being a limited number of ways of packing helices and strands in 3D space Reasons for Structural Similarity
C lass Domain structure database A Orengo & Thornton 1994 rchitecture T opology or Fold Group H omologous Superfamily ~50,000 domains in PDB ~1500 domain superfamilies in CATH
H C A T 3 Class ~36 Architecture Topology or Fold ~810 ~50,000 domains domain database
H A T C Topology or Fold Group ~810 40,000 domain entries ~50,000 domain entries Homologous Superfamily (Domain Family) ~1500 Sequence Family (35%, 60%, 95%)
DHS Dictionary of Homologous Superfamilies http://www.biochem.ucl.ac.uk/bsm/dhs Description of structural and functional characteristics for each superfamily
DHS Dictionary of Homologous Superfamilies http://www.biochem.ucl.ac.uk/bsm/dhs Description of structural and functional characteristics for each superfamily
Population of CATH Families and Structural Groups ~50,000 structural domains cluster proteins with similar sequences S ~4000 sequence families (35%) cluster proteins with similar structures and functions ~1,500 homologous superfamilies H cluster proteins with similar structures T ~810 fold groups A ~36 architectures C 3 major protein classes
Arc repressor-like Rossmann Fold OB Fold Alpha/Beta Plaits Jelly Roll CATH Arc repressor-like nearly one third of the superfamilies belong to <10 fold groups Up-down Rossmann SH3-like OB fold Immunoglobulin Jelly Roll Alpha-beta plait TIM barrel